May 13, 2013

Facial reconstruction of 5,600-year old Maltese woman

Source: Revealed...the face of a Maltese woman 5,600 years ago

Heritage Malta also launched a 3D virtual reconstruction of facial features based on one of the prehistoric skulls (over 5,000 years old) found at the Xaghra Stone Circle in Gozo. It revealed, for the very first time, what one of the earliest Maltese actually looked like.
It was a face which was much closer to what one would expect from a woman of our day and age rather than that of a person who lived on the islands over 5,000 years ago.


May 10, 2013

Links between Mycenaeans and Scandinavia

Three papers on a similar theme. An excerpt from a source mentioned in the second paper:
Det visar sig att alla undersökta svenska föremål utom ett enda - en slaggbit - kommer från gruvor och malmfyndigheter från platser på Cypern, Sardinien, Iberiska halvön, Massif Central i nuvarande Frankrike, Tyrolen samt Brittiska öarna. Kopparn har transporterats hit och i utbyte har man skeppat tillbaka stora mängder bärnsten. Fram träder en bild av en tid då internationella kontakter över stora vatten var självklarheter, och det redan cirka 2000 år innan vikingarna gav sig iväg på sina färder. [Google Translate]: It turns out that all examined Swedish subject except one - a slaggbit - comes from mines and ore deposits from sites in Cyprus, Sardinia, the Iberian Peninsula, the Massif Central in the current France, Tyrol and the British Isles. Copper has been transported, and in return it has been shipped back large amounts of amber. What emerges is a picture of a time when international contacts over large water was obvious, and there are already some 2000 years before the Vikings set off on their journeys.
From the third paper:
Both the lead isotope and chemical analyses have undoubtedly showed that the copper from the 33 Scandinavian Bronze Age artefacts diverges significantly from Scandinavian copper ores and that the copper must have been imported from elsewhere. The results furthermore indicate that there are variations in metal supply that are related to chronology, in resemblance with artefacts from Scandinavia as well as from other parts of Europe indicating analogous trade routes for copper, during the respective periods. Maritime networks and changing sources of metal seem to have been a key feature for Scandinavia in the Bronze Age.
Archaeology, Ethnology and Anthropology of Eurasia

Volume 40, Issue 2, June 2012, Pages 99–103

Grave Circle B at Mycenae in the Context of Links Between the Eastern Mediterranean and Scandinavia in the Bronze Age

I.B. Gubanov

Artifacts from royal burial graves Gamma and Omicron of grave circle B at Mycenae attest to cultural ties between the Eastern Mediterranean elite and that of the Scandinavian Early Bronze Age (mid- and late 2nd millennium BC). The appearance of the running spiral motif and representations of ships with rams in Scandinavia coincide with the beginning of the Mycenaean civilization. These facts, along with the finds of Baltic amber only in the royal burials at Mycenae but not in Crete, suggest that a principal role in the introduction of these cultural elements in Scandinavia during the Scandinavian Bronze Age (periods I–III according to Montelius) was played by the Mycenaean elite.

Link

Journal of Geography and Geology Vol 5, No 1 (2013)

The Bronze Age in SE Sweden Evidence of Long-Distance Travel and Advanced Sun Cult 

Nils-Axel Mörner, Bob G. Lind

The Bronze Age of Scandinavia (1750-500 BC) is characterized by the sudden appearance of bronze objects in Scandinavia, the sudden mass appearance of amber in Mycenaean graves, and the beginning of bedrock carvings of huge ships. We take this to indicate that people from the east Mediterranean arrived to Sweden on big ships over the Atlantic, carrying bronze objects from the south, which they traded for amber occurring in SE Sweden in the Ravlunda-Vitemölla–Kivik area. Those visitors left strong cultural imprints as recorded by pictures and objects found in SE Sweden. This seems to indicate that the visits had grown to the establishment of a trading centre. The Bronze Age of Österlen (the SE part of Sweden) is also characterized by a strong Sun cult recorded by stone monuments built to record the annual motions of the Sun, and rock carvings that exhibit strict alignments to the annual motions of the Sun. Ales Stones, dated at about 800 BC, is a remarkable monument in the form of a 67 m long stone-ship. It records the four main solar turning points of the year, the 12 months of the year, each month covering 30 days, except for month 7 which had 35 days (making a full year of 365 days), and the time of the day at 16 points representing 1.5 hour. Ales Stones are built after the same basic geometry as Stonehenge in England.

Link

Journal of Archaeological Science
Volume 40, Issue 1, January 2013, Pages 291–304

Moving metals or indigenous mining? Provenancing Scandinavian Bronze Age artefacts by lead isotopes and trace elements

Johan Ling et al.

The aim of this study is to further the discussion as to whether copper was extracted locally or imported to Sweden during the Bronze Age or if both of these practices could have coexisted. For this purpose, we have carried out lead isotope and chemical analyses of 33 bronze items, dated between 1600BC and 700BC. Among these are the famous Fröslunda shields and the large scrap hoard from Bräckan and other items from three regions in southern Sweden which are also renowned for their richness in copper ores. It is obvious from a comparison that the element and lead isotope compositions of the studied bronze items diverge greatly from those of spatially associated copper ores. Nor is there any good resemblance with other ores from Scandinavia, and it is concluded that the copper in these items must have been imported from elsewhere. The results furthermore indicate that there are variations in metal supply that are related to chronology, in agreement with other artefacts from Scandinavia as well as from other parts of Europe. Altogether these circumstances open up for a discussion regarding Scandinavia’s role in the maritime networks during the Bronze Age.

Link

Lakes in SE Arabia ~60 thousand years ago

From the paper:
From the current archaeological evidence, it seems that after MIS 5, the different lithic traditions within Arabia develop along separate trajectories, with no indication of additional input from Africa. Recent genetic evidence (Fernandes et al., 2012) also indicates that the relict distribution of minor haplogroups N1, N2 and X, reflects an ancient ancestry of these groups within the Arabian Peninsula which, the authors conclude, then spread from the Gulf region toward the Near East and Europe between 55 and 24 ka. The potential occurrence of increased humidity within the Arabian interior during MIS 3 would, therefore, have been instrumental in determining the success and trajectory of the autochthonous development of early human communities within the region at this time. Although Rosenberg et al. (2012) may be correct in their description of Arabia between ca. 75 and 10.5 ka as a natural barrier for human dispersal, it is possible that indigenous inhabitants may have persisted in environmental refugia around Arabia, such as the Gulf Oasis (e.g. Rose, 2010). The occurrence of a pluvial phase during the early stages of MIS 3, therefore, may have facilitated a range expansion of early humans previously contained within such refugia. To address these important issues, we present a multiproxy record of an early MIS 3 wet phase from a palaeolake sequence within the continental interior of SE Arabia.
Quaternary International Available online 22 February 2013

An early MIS 3 pluvial phase in Southeast Arabia: Climatic and archaeological implications

Ash Parton et al.

Climatic changes in Arabia are of critical importance to our understanding of both monsoon variability and the dispersal of anatomically modern humans (AMH) out of Africa. The timing of dispersal is associated with the occurrence of pluvial periods during Marine Isotope Stage (MIS) 5 (ca. 130–74 ka), after which arid conditions between ca. 74 and 10.5 ka are thought to have restricted further migration and range expansion within the Arabian interior. Whilst a number of records indicate that this phase of aridity was punctuated by an increase in monsoon strength during MIS 3, uncertainties regarding the precision of terrestrial records and suitability of marine archives as records of precipitation, mean that the occurrence of this pluvial remains debated. Here we present evidence from a series of relict lake deposits within southeastern Arabia, which formed at the onset of MIS 3 (ca. 61–58 ka). At this time, the incursion of monsoon rainfall into the Arabian interior activated a network of channels associated with an alluvial fan system along the western flanks of the Hajar Mountains, leading to lake formation. Multiproxy evidence indicates that precipitation increases intermittently recharged fluvial systems within the region, leading to lake expansion in distal fan zones. Conversely, decreased precipitation led to reduced channel flow, lake contraction and a shift to saline conditions. These findings are in contrast to the many other palaeoclimatic records from Arabia, which suggest that during MIS 3, the latitudinal position of the monsoon was substantially further south and did not penetrate the peninsula. Additionally, the occurrence of increased rainfall at this time challenges the notion that the climate of Arabia following MIS 5 was too harsh to permit the further range expansion of indigenous communities.

Link

Deleterious mutational load and recent population history (Simons et al. 2013)

UPDATE (Feb 28, 2014): This has now appeared in Nature Genetics.

arXiv:1305.2061 [q-bio.PE]

The deleterious mutation load is insensitive to recent population history

Yuval B. Simons, Michael C. Turchin, Jonathan K. Pritchard, Guy Sella (Submitted on 9 May 2013)

Human populations have undergone dramatic changes in population size in the past 100,000 years, including a severe bottleneck of non-African populations and recent explosive population growth. There is currently great interest in how these demographic events may have affected the burden of deleterious mutations in individuals and the allele frequency spectrum of disease mutations in populations. Here we use population genetic models to show that--contrary to previous conjectures--recent human demography has likely had very little impact on the average burden of deleterious mutations carried by individuals. This prediction is supported by exome sequence data showing that African American and European American individuals carry very similar burdens of damaging mutations. We next consider whether recent population growth has increased the importance of very rare mutations in complex traits. Our analysis predicts that for most classes of disease variants, rare alleles are unlikely to contribute a large fraction of the total genetic variance, and that the impact of recent growth is likely to be modest. However, for diseases that have a direct impact on fitness, strongly deleterious rare mutations likely do play important roles, and the impact of very rare mutations will be far greater as a result of recent growth. In summary, demographic history has dramatically impacted patterns of variation in different human populations, but these changes have likely had little impact on either genetic load or on the importance of rare variants for most complex traits.

Link

May 09, 2013

Phylogeography of Bantu languages (Currie et al. 2013)

Proc. R. Soc. B 7 July 2013 vol. 280 no. 1762 20130695

Cultural phylogeography of the Bantu Languages of sub-Saharan Africa

Thomas E. Currie et al.

There is disagreement about the routes taken by populations speaking Bantu languages as they expanded to cover much of sub-Saharan Africa. Here, we build phylogenetic trees of Bantu languages and map them onto geographical space in order to assess the likely pathway of expansion and test between dispersal scenarios. The results clearly support a scenario in which groups first moved south through the rainforest from a homeland somewhere near the Nigeria–Cameroon border. Emerging on the south side of the rainforest, one branch moved south and west. Another branch moved towards the Great Lakes, eventually giving rise to the monophyletic clade of East Bantu languages that inhabit East and Southeastern Africa. These phylogenies also reveal information about more general processes involved in the diversification of human populations into distinct ethnolinguistic groups. Our study reveals that Bantu languages show a latitudinal gradient in covering greater areas with increasing distance from the equator. Analyses suggest that this pattern reflects a true ecological relationship rather than merely being an artefact of shared history. The study shows how a phylogeographic approach can address questions relating to the specific histories of certain groups, as well as general cultural evolutionary processes.

Link

May 08, 2013

The Geography of Recent Genetic Ancestry across Europe (Ralph and Coop 2013)

This paper first came out last July on the arXiv and went through four versions there before its final form which has now appeared in PLoS Biology. It's great that its early release allowed other people to read it without having to wait for the completion of the peer review process.

I think that this is a good model: journals have the right and obligation to subject papers to close scrutiny according to their own procedures, but this process ought not interfere with the early availability of research results or the ability of anyone other than the chosen reviewers to comment on new results.

PLoS Biol 11(5): e1001555. doi:10.1371/journal.pbio.1001555

The Geography of Recent Genetic Ancestry across Europe

Peter Ralph, Graham Coop

The recent genealogical history of human populations is a complex mosaic formed by individual migration, large-scale population movements, and other demographic events. Population genomics datasets can provide a window into this recent history, as rare traces of recent shared genetic ancestry are detectable due to long segments of shared genomic material. We make use of genomic data for 2,257 Europeans (in the Population Reference Sample [POPRES] dataset) to conduct one of the first surveys of recent genealogical ancestry over the past 3,000 years at a continental scale. We detected 1.9 million shared long genomic segments, and used the lengths of these to infer the distribution of shared ancestors across time and geography. We find that a pair of modern Europeans living in neighboring populations share around 2–12 genetic common ancestors from the last 1,500 years, and upwards of 100 genetic ancestors from the previous 1,000 years. These numbers drop off exponentially with geographic distance, but since these genetic ancestors are a tiny fraction of common genealogical ancestors, individuals from opposite ends of Europe are still expected to share millions of common genealogical ancestors over the last 1,000 years. There is also substantial regional variation in the number of shared genetic ancestors. For example, there are especially high numbers of common ancestors shared between many eastern populations that date roughly to the migration period (which includes the Slavic and Hunnic expansions into that region). Some of the lowest levels of common ancestry are seen in the Italian and Iberian peninsulas, which may indicate different effects of historical population expansions in these areas and/or more stably structured populations. Population genomic datasets have considerable power to uncover recent demographic history, and will allow a much fuller picture of the close genealogical kinship of individuals across the world.

Link

May 07, 2013

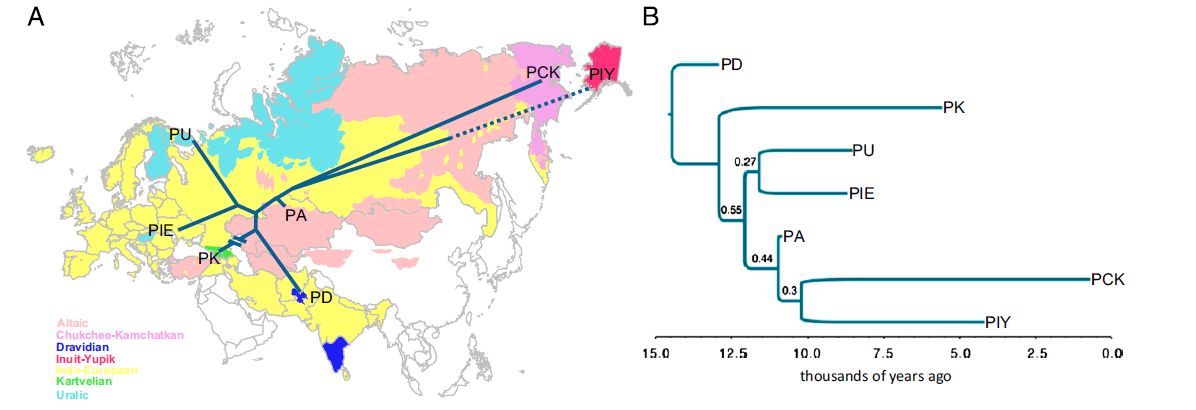
Deep common ancestry of Eurasiatic languages (Pagel et al. 2013)

From the paper:

Posterior support at internal nodes of the tree is low, as we might expect of a linguistic tree of this age, but all exceed chance expectations (SI Text) and the internal topology does not affect our estimates of the age of the superfamily. All inferred ages must be treated with caution but our estimates are consistent with proposals linking the near concomitant spread of the language families that comprise this group to the retreat of glaciers in Eurasia at the end of the last ice age ~15 kya (4, 17). The 95% CIs around the root-age are consistent with the initial separation of these families occurring before the development of agriculture beginning ~11 kya (26).

A few comments:

  • The common ancestry of Inuit-Yupik with Chukchee-Kamchatkan lends some support to the idea of Old/New World contacts postdating the initial colonization of the Americas
  • (Note that the superimposition of the tree on the map does not indicate migratory paths)
  • The deep divergence of Proto-Dravidian from the rest of the tree raises the issue of the genetic identity of the Proto-Dravidians. Today, Dravidian speakers are concentrated on the southern parts of India -with the notable Brahui exception in Pakistan- so one is tempted to associate them with the long diverged "Ancestral South Indian" genetic component whose closest living relatives live in the Indian Ocean. On the other hand, hypothesized relationships between Dravidian and extra-Indian languages, such as those postulated here might suggest that Proto-Dravidian was spoken by people more closely related to other Eurasians.
  • More generally, the hypothesis of post-glacial contacts between diverse parts of Eurasia might suggest that differentiation between Eurasian peoples did not proceed in isolation after the initial Out-of-Africa settlement. And, if there were indeed post-glacial movements, of people spreading "Proto-Eurasiatic" languages, these may be detectable by archaeogenetic means.

With the two earliest offshoots being Proto-Dravidian and Proto-Kartvelian, it would be tempting to seek some Central Asian proto-homeland for these languages; the remaining languages seem to occupy (mostly) areas that were substantially glaciated. There was of course large-scale language replacement during the Neolithic and even later time periods, so one can hypothesize that other extinct languages may also have belonged to this greater family, and it would be interesting to see if membership could be supported for any of them.

ScienceNOW has a fairly good high-level discussion. The paper is open access.

PNAS May 6, 2013, doi: 10.1073/pnas.1218726110

Ultraconserved words point to deep language ancestry across Eurasia

Mark Pagel et al.

The search for ever deeper relationships among the World’s languages is bedeviled by the fact that most words evolve too rapidly to preserve evidence of their ancestry beyond 5,000 to 9,000 y. On the other hand, quantitative modeling indicates that some “ultraconserved” words exist that might be used to find evidence for deep linguistic relationships beyond that time barrier. Here we use a statistical model, which takes into account the frequency with which words are used in common everyday speech, to predict the existence of a set of such highly conserved words among seven language families of Eurasia postulated to form a linguistic superfamily that evolved from a common ancestor around 15,000 y ago. We derive a dated phylogenetic tree of this proposed superfamily with a time-depth of ∼14,450 y, implying that some frequently used words have been retained in related forms since the end of the last ice age. Words used more than once per 1,000 in everyday speech were 7- to 10-times more likely to show deep ancestry on this tree. Our results suggest a remarkable fidelity in the transmission of some words and give theoretical justification to the search for features of language that might be preserved across wide spans of time and geography.

Link

May 02, 2013

Small-bodied humans from the Terminal Pleistocene in Tanzania

East Africa is known for the tall and lean physiques of many of its current inhabitants, but there has been speculation -on linguistic or other grounds- that it was once home to people similar to the present-day Bushmen of southern Africa. A new publication on small-bodied humans from Tanzania may be related to this hypothesis.

From the paper:
New discoveries, such as B-1 from Mlambalasi, may renew discussion on the presence of small-bodied people in East Africa. Based on the few comparable skeletal samples, this individual does not conform to the typical tall, robust, and linear body proportions of previously reported East African LSA populations. Instead, itssmall body size has more in common with southern African peoples. This does not necessarily imply a biological link between these LSA populations. Hypotheses for why small size develops include the need for thermoregulation, limited food supply, enhanced mobility, and high mortality influencing early reproduction (Perry and Dominy, 2009; Pfeiffer and Harrington, 2011). In southern Africa, small body size may be linked to energetics and accident avoidance. The rate of injury among the South African LSA populations is lower than other mobile hunter-gatherer groups, which Pfeiffer (2007) interprets as possibly related to reduced body mass. Ethnographic studies of modern Khoesan emphasize the centrality of the bow and arrow and persistence hunting, in which small, energetically efficient bodies prove advantageous (Tobias, 1978). Small body size may have emerged multiple times, perhaps amidst the low population densities and climatic instability of the LSA. Given that early modern humans may have endured a population crisis (Harpending et al., 1993; Ambrose, 1998a; Lahr and Foley, 1998; Reich and Goldstein, 1998), and that there is some evidence for increased diversity among earlier populations (Crevecoeur et al., 2009), one characteristic of some terminal Pleistocene and early Holocene groups may have been a small body size. Exploring the incidence of scope of this pattern in East African and other early modern humans may shed light on the importance of body size in human evolution.

International Journal of Osteoarchaeology DOI: 10.1002/oa.2323

Terminal Pleistocene Later Stone Age Human Remains from the Mlambalasi Rock Shelter, Iringa Region, Southern Tanzania†

E. A. Sawchuk1, P. R. Willoughby

This paper introduces research at the Mlambalasi rock shelter in the Iringa Region of southern Tanzania. The deposits are composed of a historic and Iron Age occupation, a microlithic Holocene Later Stone Age (LSA), and then a macrolithic Late Pleistocene LSA. Middle Stone Age deposits are also present on the slope in front of the rock shelter. Excavations in A.D. 2002, 2006, and 2010 yielded fragmentary human remains as well as pottery, iron, stone tools, faunal bone, and glass and ostrich eggshell beads. Among the human remains, four individuals are present: two adults and a juvenile were found in the same LSA context, and another adult associated with the Iron Age/historic period. The most complete skeleton is an adult of indeterminate sex that was found in situ in an LSA deposit. Charcoal in proximity to the bone was AMS radiocarbon dated to 12,925 cal BC (OxA-24620), which is consistent with radiocarbon dates on giant land snail shells from above and below the remains. The skeleton exhibits a series of pathological changes such as extensive dental wear and carious lesions, as well as damage most likely caused by termites, post-mortem. The most striking aspect of this individual is its small size; stature and body mass estimations place it in the range of historic Khoesan from southern Africa. Consequently, this research adds to the discourse regarding the existence of small-bodied people in the East African LSA. Findings from this new skeletal sample will contribute to studies of human biology and variation in Africa during the terminal Pleistocene and Holocene. This article is protected by copyright. All rights reserved.

Link

April 29, 2013

Okhotsk and Ainu: linguistic connection?

A genetic connection was hypothesized in the third of the following related links on the basis of ancient Jomon mtDNA that seemed to lack an element of the modern Ainu gene pool.

From the current paper:
If we accept a view that transmission of language may be gender-specific [50]–[52], then we are able to formulate at least two hypotheses for the specific processes of the Ainu language origin. Because Y-chromosome haplogroup D is thought to represent Jomon male ancestry, the predominance of that particular haplogroup in the Ainu (75–87.5%) implies that the majority of Ainu male ancestry is from the Jomon [53], [54], whereas a heavy mixture of mtDNA haplogroups indicates that a significant proportion of the Ainu female ancestry is from the Okhotsk (excluding 35.3% of mtDNA haplogroups that the Ainu share with other neighboring populations, 39.4% of the remaining female heritage is shared exclusively with the Okhotsk and the rest is a mixture of both Jomon and Okhotsk [18], [47], [54]). If we thus assume male-specific language transmission for the Ainu, the first hypothesis for the processes behind the Ainu language origin could be that proto-Ainu arose from a large number of Jomon males who intermarried with Okhotsk females in northern Hokkaido, and subsequently spread to the rest of region. Similarly, if we assume that the transmission of Ainu language corresponds with female ancestry, the second hypothesis could be that proto-Ainu was spoken by the incoming Okhotsk females who merged with the preexisting Jomon males. Based on these observations, we propose that one potential way of understanding how language change occurred for the Ainu is to estimate which gender was more influential when early Ainu people established family membership. This may be carried out indirectly by revealing the signature of historical post-marital residence pattern via estimating the degrees of genetic variation in their Y-chromosome and mtDNA [55] as well as reconstructing ancestral post-marital residence rules from regional cultural variation [56]. Investigating which model of language change [57] is relevant to the Ainu is a direction that deserves more attention, and acquiring an accurate description of how language change occurred for the Ainu would allow us to make further inferences about the deeper history of the human lineage that once thrived in northern Japan.
I would think that a fairly recent major event of Okhotsk+Jomon=Ainu would be detectable both by ancient DNA analysis and by the study of the modern Ainu. It is certainly fascinating that the Ainu rather than being a bona fide relic of the earliest inhabitants of Japan may actually have complex ancestry themselves, and in the very recent past at that.

Related:

  1. Craniometry of the Ainu
  2. Metric and non-metric variation of Ainu
  3. Ancient mtDNA of Hokkaido Jomon
  4. Ainu/Ryukyuan paper

Evolution of the Ainu Language in Space and Time

Sean Lee, Toshikazu Hasegawa

Languages evolve over space and time. Illuminating the evolutionary history of language is important because it provides a unique opportunity to shed light on the population history of the speakers. Spatial and temporal aspects of language evolution are particularly crucial for understanding demographic history, as they allow us to identify when and where the languages originated, as well as how they spread across the globe. Here we apply Bayesian phylogeographic methods to reconstruct spatiotemporal evolution of the Ainu language: an endangered language spoken by an indigenous group that once thrived in northern Japan. The conventional dual-structure model has long argued that modern Ainu are direct descendants of a single, Pleistocene human lineage from Southeast Asia, namely the Jomon people. In contrast, recent evidence from archaeological, anthropological and genetic evidence suggest that the Ainu are an outcome of significant genetic and cultural contributions from Siberian hunter-gatherers, the Okhotsk, who migrated into northern Hokkaido around 900–1600 years ago. Estimating from 19 Ainu language varieties preserved five decades ago, our analysis shows that they are descendants of a common ancestor who spread from northern Hokkaido around 1300 years ago. In addition to several lines of emerging evidence, our phylogeographic analysis strongly supports the hypothesis that recent expansion of the Okhotsk to northern Hokkaido had a profound impact on the origins of the Ainu people and their culture, and hence calls for a refinement to the dual-structure model.

Link

April 24, 2013

Criticism of Y-chromosome Adam old age

... has just appeared on the arXiv. This refers to the paper by Mendez et al. announcing the basal clade A00 of the phylogeny and estimating a TMRCA for Y-chromosome Adam of 237-581ka.

The author argues that such an old age is inconsistent with neutral theory, although that assumes no population structure in the origin of modern humans; it may very well be that A00 introgressed into the modern human gene pool via an admixture event from a different African population.

The best evidence for the authors' of the original paper choice of mutation rate is their estimate that the common ancestor of all Eurasians being ~63ky vs. ~39ky using the faster rate. While a date between these two can be probably accommodated, the ~39ky age seems difficult to accept, given that Homo sapiens had arrived in various parts of Eurasia by the mid-40ky's and had been admixing with Neandertals 47-65ky BP; a higher date would also be more in line with age estimates of Eurasian mtDNA macro-haplogroups M and N.

In any case, it's probably a good idea to get a better handle on the mutation rate: Mendez et al. rely on the autosomal rate, adjusting for the Y-chromosome; while the faster rate derives from a single Chinese deep pedigree study.

arXiv:1304.6098 [q-bio.PE]

Timing of ancient human Y lineage depends on the mutation rate: A comment on Mendez et al

Melissa A. Wilson Sayres (Submitted on 22 Apr 2013)

Mendez et al. recently report the identification of a Y chromosome lineage from an African American that is an outgroup to all other known Y haplotypes, and report a time to most recent common ancestor, TMRCA, for human Y lineages that is substantially longer than any previous estimate. The identification of a novel Y haplotype is always exciting, and this haplotype, in particular, is unique in its basal position on the Y haplotype tree. However, at 338 (237-581) thousand years ago, kya, the extremely ancient TMRCA reported by Mendez et al. is inconsistent with the known human fossil record (which estimate the age of anatomically modern humans at 195 +- 5 kya), with estimates from mtDNA (176.6 +- 11.3 kya, and 204.9 (116.8-295.7) kya) and with population genetic theory. The inflated TMRCA can quite easily be attributed to the extremely low Y chromosome mutation rate used by the authors.

Link

mtDNA haplogroup H and the origin of Europeans (Brotherton et al. 2013)

Panel b is particularly interesting, as it clearly shows the Iberian-ness of Bell Beaker mtDNA (BBC), and the South-Eastern-ness of LBK.

From the paper:
From around 2800 BC, the LNE Bell Beaker culture emerged from the Iberian Peninsula to form one of the first pan-European archaeological complexes. This cultural phenomenon is recognised by a distinctive package of rich grave goods including the eponymous bell-shaped ceramic beakers. The genetic affinities between Central Europe’s Bell Beakers and present-day Iberian populations (Fig. 2) is striking and throws fresh light on long-disputed archaeological models3. We suggest these data indicate a considerable genetic influx from the West during the LNE. These far-Western genetic affinities of Mittelelbe-Saale’s Bell Beaker folk may also have intriguing linguistic implications, as the archaeologically-identified eastward movement of the Bell Beaker culture has recently been linked to the initial spread of the Celtic language family across Western Europe39. This hypothesis suggests that early members of the Celtic language family (for example, Tartessian)40 initially developed from Indo-European precursors in Iberia and subsequently spread throughout the Atlantic Zone; before a period of rapid mobility, reflected by the Beaker phenomenon, carried Celtic languages across much of Western Europe. This idea not only challenges traditional views of a linguistic spread of Celtic westwards from Central Europe during the Iron Age, but also implies that Indo-European languages arrived in Western Europe substantially earlier, presumably with the arrival of farming from the Near East41.
It does seem increasingly likely that there was a major Out-of-Iberia episode which may very well have involved a population of relative newcomers (R1b males, undetected in Europe in the pre-5ka period) interacting with an "Iberian" matrilineal substratum and then exporting both R1b and the "Iberian" type of H into most of Western Europe with the Bell Beaker phenomenon. It's hard to think of the Bell Beakers as ultimately descended from the first farmers alone, both because of their distinctive physical type, and also because of the aforementioned absence of R1b in early farmers. More ancient DNA work will certainly help solve many of the remaining puzzles.

Also from the paper:
The demographic reconstruction, which is based on direct calibration points, has major implications for understanding post-glacial human history in Europe. Our new estimate is incompatible with traditional views that the majority of present-day hg H lineages were carried into Central, Northern and Eastern Europe via a post-glacial human population expansion before the Holocene (12 kya)13. Our data complement a recent study, based on present-day mt genomes, which describes a pronounced population increase at ~7000 BC (interpreted as a Neolithic expansion into Europe), but followed by a slow population growth until the present day26. By including ancient DNA data from across the critical time points in question, our skyride plot corrects for missing temporal data and suggests substantial growth of hg H from the beginning of the Neolithic and continuing throughout the entire Neolithic period. This emphasizes the role of farming practices and cultural developments in the demographic expansions inferred in subsequent time periods, which have not yet been explored genetically.
Nature Communications 4, Article number: 1764 doi:10.1038/ncomms2656

Neolithic mitochondrial haplogroup H genomes and the genetic origins of Europeans

Paul Brotherton et al.

Haplogroup H dominates present-day Western European mitochondrial DNA variability (>40%), yet was less common (~19%) among Early Neolithic farmers (~5450 BC) and virtually absent in Mesolithic hunter-gatherers. Here we investigate this major component of the maternal population history of modern Europeans and sequence 39 complete haplogroup H mitochondrial genomes from ancient human remains. We then compare this ‘real-time’ genetic data with cultural changes taking place between the Early Neolithic (~5450 BC) and Bronze Age (~2200 BC) in Central Europe. Our results reveal that the current diversity and distribution of haplogroup H were largely established by the Mid Neolithic (~4000 BC), but with substantial genetic contributions from subsequent pan-European cultures such as the Bell Beakers expanding out of Iberia in the Late Neolithic (~2800 BC). Dated haplogroup H genomes allow us to reconstruct the recent evolutionary history of haplogroup H and reveal a mutation rate 45% higher than current estimates for human mitochondria.

Link

April 17, 2013

Y-chromosomes of Native South Americans (Roewer et al. 2013)

It would be useful to sequence these South American C3* Y-chromosomes to see how they are related to the C3b-P39 found in some native North Americans as well as other unresolved C3* from Asia. It would also be worthwhile to look at autosomal data from these populations, to see if they are wholly descended from First Americans, or have evidence of more recent gene flow from East Asia.

PLoS Genet 9(4): e1003460. doi:10.1371/journal.pgen.1003460

Continent-Wide Decoupling of Y-Chromosomal Genetic Variation from Language and Geography in Native South Americans

Lutz Roewer et al.

Numerous studies of human populations in Europe and Asia have revealed a concordance between their extant genetic structure and the prevailing regional pattern of geography and language. For native South Americans, however, such evidence has been lacking so far. Therefore, we examined the relationship between Y-chromosomal genotype on the one hand, and male geographic origin and linguistic affiliation on the other, in the largest study of South American natives to date in terms of sampled individuals and populations. A total of 1,011 individuals, representing 50 tribal populations from 81 settlements, were genotyped for up to 17 short tandem repeat (STR) markers and 16 single nucleotide polymorphisms (Y-SNPs), the latter resolving phylogenetic lineages Q and C. Virtually no structure became apparent for the extant Y-chromosomal genetic variation of South American males that could sensibly be related to their inter-tribal geographic and linguistic relationships. This continent-wide decoupling is consistent with a rapid peopling of the continent followed by long periods of isolation in small groups. Furthermore, for the first time, we identified a distinct geographical cluster of Y-SNP lineages C-M217 (C3*) in South America. Such haplotypes are virtually absent from North and Central America, but occur at high frequency in Asia. Together with the locally confined Y-STR autocorrelation observed in our study as a whole, the available data therefore suggest a late introduction of C3* into South America no more than 6,000 years ago, perhaps via coastal or trans-Pacific routes. Extensive simulations revealed that the observed lack of haplogroup C3* among extant North and Central American natives is only compatible with low levels of migration between the ancestor populations of C3* carriers and non-carriers. In summary, our data highlight the fact that a pronounced correlation between genetic and geographic/cultural structure can only be expected under very specific conditions, most of which are likely not to have been met by the ancestors of native South Americans.

Link

April 12, 2013

Haplotype that looks Neandertal-introgressed may reflect African population structure (Gokcumen et al. 2013)

From the paper:
Several scenarios can be envisioned to explain the unusual genetic variation observed at the NE1 locus: (1) recent Neandertal admixture exclusively with Eurasian populations, (2) back migration to Africa from Eurasia after Neandertal admixture with Eurasian populations, and (3) ancient African substructure maintained since before Human-Neandertal divergence (Figure 3A). 
...
The presence of African NE1 haplotypes does not support the first scenario of exclusive Neandertal admixture with Eurasian populations. Recent reports have suggested that Neandertals and Denisovans contributed their genetic material to present-day Eurasian populations and Melanesians, respectively [20], [21]. However, the variation that we observe at the NE1 locus is not consistent with direct archaic hominin admixture as discussed in these publications. We did not consider Neandertal admixture into ancient African populations because of paleoanthropological studies that only report interactions between Neandertals and modern humans outside of Africa [37].
Thinking about the last sentence, paleoanthropological studies only report interactions between Neandertals and modern humans in "parts of outside Africa", but the signal of Neandertal admixture exists all over "outside Africa". It is not incoceivable that Neandertal-admixed Eurasians back-migrated into Africa and introduced NE1 to African populations. Such hypothetical back-migrants would not appear Neandertaloid in tha paleoanthropological sense. The authors consider this possibility:
The second scenario assumes back migration into Africa from Eurasian populations after the admixture of Neandertal with Eurasian populations [38]. If such admixture occurred, the African NE1 haplotypes should represent a subset of Eurasian NE1 haplotypes. To test this, we again analyzed the phase 1 data of the 1000 Genomes Project, which includes 338 haplotypes from three African populations. Using this dataset, we found that variation within African NE1 haplotypes is significantly higher than variation within Asian and European NE1 haplotypes (p less than 10-15, Figure 3C, Figure S5). This result indicates that African NE1 haplotypes have a longer coalescence and, as such, the presence of the NE1 haplogroup among modern Africans cannot be explained by simple back migration and admixture of Eurasian haplotypes to African populations.
But, it is possible that the higher variation within African NE1 haplotypes may reflect introgression of short "Palaeoafrican" variants within the African NE1 haplotypes. Such variants would appear as excess variation, but would not be "provable" as introgression in the absence of a comparative archaic African genome. This is a recurring theme, that (part of?) the African-Eurasian diversity differential can be explained both in terms of loss of diversity in an Out-of-Africa bottleneck and a gain-of-diversity in In-Africa admixture events between divergent populations that must have lived in the large and ecologically diverse continent. Which brings us to scenario #3:

The third scenario represents the persistence of an old African substructure at the NE1 locus before the Human-Neandertal divergence (Figure 3A). This scenario explains the presence of NE1 haplotypes (that are similar to the Neandertal haplotype) among modern human populations as well as the deep, distinct lineages observed among African NE1 haplotypes. To corroborate this conclusion, we estimated the coalescence of NE1 haplotypes through network analysis (Figure S6) and found a coalescence time of between ~437 K and ~993 K years before present (YBP) for African NE1 haplotypes and ~134 K YBP and ~304 K YBP for European NE1 haplotypes. These observations collectively suggest that the most parsimonious explanation for the observed variation at the NE1 locus is that the NE1/nonNE1 haplogroups arose after the human-chimpanzee common ancestor, but before the Human-Neandertal split in Africa. As such, the variation at the NE1 locus has persisted within ancient African substructure and later spread to non-African populations.


  PLoS Genet 9(4): e1003404. doi:10.1371/journal.pgen.1003404

Balancing Selection on a Regulatory Region Exhibiting Ancient Variation That Predates Human–Neandertal Divergence

Omer Gokcumen et al.

Ancient population structure shaping contemporary genetic variation has been recently appreciated and has important implications regarding our understanding of the structure of modern human genomes. We identified a ~36-kb DNA segment in the human genome that displays an ancient substructure. The variation at this locus exists primarily as two highly divergent haplogroups. One of these haplogroups (the NE1 haplogroup) aligns with the Neandertal haplotype and contains a 4.6-kb deletion polymorphism in perfect linkage disequilibrium with 12 single nucleotide polymorphisms (SNPs) across diverse populations. The other haplogroup, which does not contain the 4.6-kb deletion, aligns with the chimpanzee haplotype and is likely ancestral. Africans have higher overall pairwise differences with the Neandertal haplotype than Eurasians do for this NE1 locus (p less than 10-15). Moreover, the nucleotide diversity at this locus is higher in Eurasians than in Africans. These results mimic signatures of recent Neandertal admixture contributing to this locus. However, an in-depth assessment of the variation in this region across multiple populations reveals that African NE1 haplotypes, albeit rare, harbor more sequence variation than NE1 haplotypes found in Europeans, indicating an ancient African origin of this haplogroup and refuting recent Neandertal admixture. Population genetic analyses of the SNPs within each of these haplogroups, along with genome-wide comparisons revealed significant FST (p = 0.00003) and positive Tajima's D (p = 0.00285) statistics, pointing to non-neutral evolution of this locus. The NE1 locus harbors no protein-coding genes, but contains transcribed sequences as well as sequences with putative regulatory function based on bioinformatic predictions and in vitro experiments. We postulate that the variation observed at this locus predates Human–Neandertal divergence and is evolving under balancing selection, especially among European populations.

Link

April 10, 2013

Closed-access story about DIY analysis tools

I find it a little odd that this story about DIY analysis tools, which (apparently) includes some quotes by myself, has now appeared in a closed-access publication. Had I known that to be the case, I doubt that I would have offered any response. It's probably not too late to make that item open access. 

In any case here's what I had to say (in full) to the author of the piece:

I think that a plurality of tools from a number of different analysts is an unambiguously good thing, both for the creators of these tools and their users.

For the users it is good because they can obtain different assessments of their ancestry, so they learn to be skeptical of extraordinary or unexpected claims of any particular test, and also to be more convinced of results that recur across many different tests.

For the creators it is good because of both (i) the motivation to improve their tools driven by competition with other test creators, and also (ii) the feedback they get from users of their tests.

These tools are also good for science in general, because a plurality of eyes (test creators and users) examine genetic data trying to detect interesting patterns in them that might be missed by more narrowly-focused research. So, a whole ecosystem of ideas springs up from these tests, as people try to fit their results into a broader pattern of human history. This is complementary to academic research: less structured and more "noisy" in terms of ideas that don't pan out, but also more dynamic, fast-paced and democratic.

As for Dodecad, I have developed my calculators by utilizing standard population genetics software, as well as software developed by myself, making use of publicly accessible academic datasets together with data from volunteers; the latter is very useful, because it helps me fill in gaps in population coverage: either because some populations have not been sampled in the literature yet, or, if they have, because their data is not publicly accessible to everyone.

Pottery-using hunter-gatherer cooks from Japan

From an accompanying piece:
Pottery usage among hunter-gatherers was considered somewhat anomalous and counter-intuitive; fragile pots did not seem to have a place in the mobile lifestyles thought to characterize most human existence before the advent of farming villages during the Neolithic, from about 10,000 years ago in the eastern Mediterranean. But the discovery of lipids on ceramic vessels in East Asia dating from the Late Pleistocene, about 15,000–12,000 years ago, presented by Craig et al.2 in a paper published on Nature's website today, suggests that some hunter-gatherers used pots for cooking. The report also provides a demonstration of how science should be integral to our piecing together of history. 
... 
Our knowledge that ceramic containers were being made and used by hunter-gatherers in the Late Pleistocene in various parts of East Asia — from Japan to far eastern Russia and north and south China — means that pottery usage among hunter-gatherers is no longer seen as anomalous in the Old World. In fact, there may be evidence for routes of the introduction of pottery into Europe that are not associated with the introduction of farming13.
From the paper itself:
From both the bulk stable isotope data and the more specific product identifications based on available lipid data, we suggest that aquatic products were the most frequently processed products in Incipient Jōmon pottery, through the fluctuating climate and across a range of environments, from Hokkaido in the north to Kyushu in the south. Whether ceramic vessels were integral to the processing of aquatic resources or, as is suggested by their rarity, were used only occasionally, perhaps ceremonially or as a prestige technology24, remains debatable.
Nature (2013) doi:10.1038/nature12109

Earliest evidence for the use of pottery 

O. E. Craig et al.


Pottery was a hunter-gatherer innovation that first emerged in East Asia between 20,000 and 12,000 calibrated years before present1, 2 (cal BP), towards the end of the Late Pleistocene epoch, a period of time when humans were adjusting to changing climates and new environments. Ceramic container technologies were one of a range of late glacial adaptations that were pivotal to structuring subsequent cultural trajectories in different regions of the world, but the reasons for their emergence and widespread uptake are poorly understood. The first ceramic containers must have provided prehistoric hunter-gatherers with attractive new strategies for processing and consuming foodstuffs, but virtually nothing is known of how early pots were used. Here we report the chemical analysis of food residues associated with Late Pleistocene pottery, focusing on one of the best-studied prehistoric ceramic sequences in the world, the Japanese Jomon. We demonstrate that lipids can be recovered reliably from charred surface deposits adhering to pottery dating from about 15,000 to 11,800?cal?BP (the Incipient Jomon period), the oldest pottery so far investigated, and that in most cases these organic compounds are unequivocally derived from processing freshwater and marine organisms. Stable isotope data support the lipid evidence and suggest that most of the 101 charred deposits analysed, from across the major islands of Japan, were derived from high-trophic-level aquatic food. Productive aquatic ecotones were heavily exploited by late glacial foragers3, perhaps providing an initial impetus for investment in ceramic container technology, and paving the way for further intensification of pottery use by hunter-gatherers in the early Holocene epoch. Now that we have shown that it is possible to analyse organic residues from some of the world’s earliest ceramic vessels, the subsequent development of this critical technology can be clarified through further widespread testing of hunter-gatherer pottery from later periods.

Link